
Tomato (Lycopersicon esculentum Mill.) is a globally remarkable crop, yet its production is severely limited by fungal pathogens that cause fruit rots, particularly those caused by Alternaria species. The aims of this study were to evaluate several integrated and eco-friendly strategies for the management of tomato fruit rot and assess their effectiveness in improving yield, fruit quality, and key biochemical attributes. Fungal diseases considerably contribute to substantial losses in tomato fruits throughout handling, storage, and distribution from harvest to the consumer. In this study, several fungi originating from rotten tomato fruits in Menoufia Governorate, Egypt, were isolated and identified as A. solani and A. alternata, where A. solani was more prevalent and virulent, causing severe early blight symptoms, particularly in the Super strain B hybrid (recording 96.30% incidence and 34.36% severity). Several biocontrol agents, including Trichoderma album, T. atroviride, T. harzianum, T. viride, and the commercial product Blight Stop (T. harzianum) exhibited a strong in vitro antagonistic activity against A. solani, with T. album achieving the highest inhibition (90.28%). In vivo, all bio-agents and Blight Stop reduced disease incidence and severity of tomato fruit rot, with T. album achieving the greatest control efficiency, recording 73.56% and 74.76% during 2023/24–2024/25 growth seasons, respectively, followed by T. atroviride and Blight Stop. Additionally, these treatments enhanced multiple yield components, including fruit quality (total soluble solids “TSS”, vitamin C, protein content, carbohydrates), and several other biochemical traits such as flavonoids and phenolics content, and defense-related enzymes (i.e., peroxidase (PO), polyphenol oxidase (PPO), chitinase, and β-1,3-glucanase), with T. album consistently recorded the highest values. These findings highlight the effectiveness of Trichoderma spp. as biocontrol agents and promising alternatives to chemical pesticides for suppressing post-harvest tomato diseases and improving plant performance, thereby underscoring their potential as sustainable and ecofriendly tools for disease management.
Research Article · Volume 10, Issue 5, 8 September 2026 · Open Access
Efficacy of Trichoderma species as Biocontrol Agents for Management of Tomato Fruit Rot
· · · ·
Affiliations & Notes ⌄
- 1Central Laboratory of Organic Agriculture (CLOA), Agricultural Research Center (ARC), Giza, Egypt
- 2Plant Pathology Research Institute, Agricultural Research Center (ARC), Giza, Egypt
- 3Faculty of Agriculture, Cairo University, Egypt
- 4Faculty of Agriculture, Benha University, Benha, Egypt. *Correspondence | Mohamed F.A. Ahmed, Central Laboratory of Organic Agriculture (CLOA), Agricultural Research Center (ARC), Giza, Egypt
- 5Email: mohamed_faah@yahoo.com
Article Info ⌄
- Journal:
- Novel Research in Microbiology Journal
- Published:
- 8 September 2026
From the article
- The present field results clearly demonstrated that all tested Trichoderma spp. based treatment’s considerably reduced tomato fruit rot compared to the untreated control, confirming their effectiveness as biological control agents under natural conditions.
- All Trichoderma spp. and Blight stop-based treatments considerably increased flavonoid and total phenolic contents in tomato leaves compared to the untreated control, indicating an enhanced plant defense and antioxidant capacity across both seasons.
- This study demonstrated the potential of integrated, eco-friendly biocontrol strategies for managing tomato fruit rot while improving yield, fruit quality, and plant defense responses.
- Based on the present findings, T. album is recommended as a promising eco-friendly biocontrol agent for the integrated management of tomato fruit rot caused by Alternaria solani.
Selected from the article's own text.
Abstract
Introduction
Tomato (Lycopersicon esculentum Mill.) is a globally important crop and a key component of Egyptian agriculture, with over 153,000 hectares cultivated and about 6.7 million tons produced annually ; FAO, 2024). However, its production is heavily constrained by fungal diseases such as fruit rots, early blight, and wilts, which account for over 50% of yield losses ; ; . Due to the environmental and health risks of the chemical fungicides, use of biological control agents has emerged as a sustainable alternative for disease management ; . Trichoderma spp. (e.g., T. album, T. atroviride, T. harzianum, T. viride, and Blight stop) effectively controlled tomato fruit rot caused by Alternaria spp. through mycoparasitism, antibiosis, competition, and induced systemic resistance, with T. harzianum showing the highest efficacy ; ; ; . Additionally, these treatments enhanced yield and fruit quality (i.e., total soluble solids TSS, vitamin C, protein content, and carbohydrates content) by improving plant growth and metabolic activity ; ; . They also stimulated several biochemical defenses, including increased phenolics, flavonoids, and activity of defense enzymes such as peroxidase (PO), polyphenol oxidase (PPO), chitinase, and β-1,3-glucanase, with T. harzianum consistently induced the strongest responses ; . Additionally, T. viride acts as a biofungicide against multiple soil- and fruit-borne pathogens . Trichoderma spp. promote plant growth and immune response by producing secondary metabolites and defense-related enzymes, including chitinase, PO, and PPO, which increase resistance to microbial infections ; ; . The objectives of this study were to assess several integrated and ecofriendly strategies for managing tomato fruit rot, and enhancing yield, fruit quality, and key biochemical attributes.
Materials and Methods
Tomato cultivars
Five tomato hybrid varieties, mainly Super Strain B, Super Strain B Regular, Eliza, Castle Rock, and Super Altery were obtained from the Vegetable Research Department, Horticulture Research Institute, Agricultural Research Centre (ARC), Giza, Egypt to evaluate their susceptibility to tomato fruit rot post-harvest disease.
Isolation and identification of the tomato early blight pathogen
During autumn 2023, 100 infected tomato leaves showing early blight symptoms were collected from fields of Menoufia Governorate, Egypt, representing different tomato cultivars, including Super Strain B, Super Strain B Regular, Eliza, and Castle Rock. Infected tissues were cut into small pieces (≈2 mm) using a disinfected scissor, surface sterilized with 0.5% NaOCl for 2–3 min, rinsed three times with sterile distilled water, and air dried before being aseptically placed onto the surface of Potato Dextrose Agar (PDA) plates . Ten plates were used, each containing five pieces of infected leaf tissue. The inoculated plates were incubated at 25 ± 2 °C under a 12-h light/12-h dark photoperiod for 7 d. After incubation, the developed fungal hyphae were picked, purified using single spore colony technique, sub-cultured on PDA slants, and stored at 5–10°C for further study. The isolated fungi were identified based on their morphological characteristics according to several standard keys described by Singh (1982); Barnett and Hunter (1987); Simmons (2007).
Pathogenicity tests
Preparation of Alternaria sp. inoculum
Alternaria sp. was cultured on PDA plates at 27°C under a 12 h light/dark cycle for 15 d . Conidia were collected by adding 5 ml sterile distilled water and scraping the culture with a sterile spatula. The inoculum was adjusted to 5×10⁶ spores/ml using a haemocytometer .
Greenhouse experiment
The study was conducted in 2024 at ARC greenhouse facilities, Egypt. Five tomato hybrids were tested for their susceptibility to A. solani. Seedlings of tomato were transplanted into steam-sterilized soil in pots each containing 2.7 kg of light clay soil, with three seedlings per pot. Each replicate consisted of 30 seedlings distributed among 10 pots. Plants were spray inoculated using a hand-held atomizer with 30 ml of the prepared spore suspension, whereas control seedlings were sprayed with 30 ml of sterile distilled water. Three replicates were maintained for each tomato hybrid.
Disease assessment
After inoculation, the seedlings were covered with plastic bags for 48 h to maintain high humidity and grown under normal conditions in a completely randomized design. Disease severity was evaluated after two weeks using a 0–9 scale based on the infected leaf area . The standard disease severity (%) was evaluated according to the following formula:
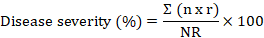
Where: n = Number of infected leaves on the plant; N= Total number of leaves examined; r = Numerical rate of infected leaves, and R= Highest numerical rate.
Biocontrol agents
Four biocontrol agents (BCAs), Trichoderma album, T. atroviride, T. harzianum, and T. viride were provided by the Biological Control Production Unit, Central Laboratory of Organic Agriculture (CLOA), Agricultural Research Centre (ARC), Giza, Egypt.
Laboratory assays
In vitro antagonistic activity
The antagonistic agents i.e., Trichoderma album, T. atrovirde, T. harzianum, T. viride, and Blight stop (T. harzianum) were individually added at the rate of 10 ml to 125 ml to conical flasks each containing 90 ml PDA before solidification, resulting in a final concentration of 10% (v/v). A disc of A. solani was cut individually from each actively growing culture using a sterile cork borer and aseptically placed at the center of each seeded plate. Control plates were inoculated with A. solani only. Each treatment was replicated three times and the plates were incubated at 25±2 °C . Incubation continued until full growth of the fungal pathogen in the control plates. The in vitro antagonistic efficacy was evaluated by calculating the percentage reduction in radial mycelial growth compared to the control, following the standard method reported by Ahmed (2013).
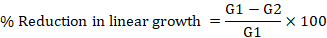
Where; G1: Growth of the pathogenic fungus in the control plates, G2: Growth of the pathogen in the treatment plates.
Field experiments
Inocula preparation of the fungal biocontrol agents
The BCAs were cultured on Gliotoxin fermentation (GF) broth medium and incubated for 10 d at 25 ± 2 °C under dark conditions to promote propagule production , 2013). After incubation, each broth culture was homogenized using an electric blender for 2 min, to obtain a uniform suspension, and the propagule concentration was adjusted to approximately 30 × 10⁶ propagule/ml. Inoculum of each bio-agent was applied at the rate of 1 L per 50 L of water.
Biofungicide
Blight Stop, a biocidal formulation containing a wild isolate of T. harzianum (30 × 10⁶ cfu/ml) was used for comparison with the tested fungal BCAs. It was applied at a rate of 1 L per 50 L of water and provided by the Biological Control Production Unit, Central Laboratory of Organic Agriculture (CLOA), ARC.
Field study setup
Field trials were conducted in Sadat City, Menoufia Governorate, Egypt, over two seasons (2023/2024 and 2024/2025) to evaluate an ecofriendly method used for managing tomato fruit rot. Tomato fruit-rot pathogen was naturally present in the used soil. Experiments used three replicated plots in a completely randomized block design, each plot measuring 112.5 m² with three ridges (25 × 1.5 m) separated by 50 cm . Tomato seeds (Super Strain B hybrid) were sown in a nursery foam tray on 1st September and grown seedlings with 3–4 true leaves were transplanted 45 d later on 15th October . Each ridge received 50 transplants of the Super Strain B hybrid, identified as highly susceptible to fruit rot based on prior pathogenicity tests. During the 2023/2024 and 2024/2025 growing seasons, composts were applied to the field soil at 1.2 kg/m² and irrigated daily. After 15 d, Super Strain B tomato transplants were planted .
Treatment of seedlings
Sixty-day-old seedlings were subjected to preharvest individual treatment using diluted (1:50) suspensions of T. album, T. atroviride, T. harzianum, and T. viride (30 × 10⁶ cfu\ml). The commercial biofungicide Blight Stop (Trichoderma spp.) was applied individually and supplemented with 5% Arabic gum and 5% potassium soap to enhance adhesion, where the mixture was allowed to stand for 10 min. prior to application . Treatments were applied as foliar sprays twice at 21-d intervals, starting on 1st of November during the 2023/2024 and 2024/2025 growing seasons, while untreated plants served as the control . Each treatment had three replicated plots, each consisting of three ridges, with a regular drip irrigation and standard organic practices. Field conditions were approximately 25 ± 5°C with 60 ± 10% relative humidity.
Disease assessment and different crop parameters
Data collection
At the end of each growing season, three plants were randomly sampled from each plot for laboratory analysis. Recorded parameters included fruit rot disease incidence, plant survival after 90 d of transplanting, and disease severity assessed 28 d after treatment .
Disease severity (DS %) was measured using the scale of Poly and Srikanta (2022) and calculated as follows:
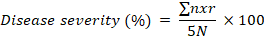
Where n is the number of plants in each rating, r is the maximum rating (5), and N is the total number of plants.
The percentages of disease incidence and efficacy of each bio-agent were calculated according to Ahmed et al. (2023); Shi et al. (2023) using the following equations:
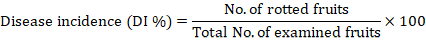
Also, % efficacy for each bio-agent was calculated as follows:

Different agricultural measures and analyses
Yield measurements
Yield components were assessed by recording the number of fruits per plant, average fruit weight (g/fruit), and total fruit yield (g/plant) from three randomly selected replicate per treatment .
Total proteins content
Total protein content was determined in tomato leaf tissues collected from three randomly selected plants per treatment, with each plant representing one biological replicate. Protein content was measured using the Bradford (1976) method.
Vitamin C content
Vitamin C content was determined in tomato fruits collected from three randomly selected plants per treatment, with each plant representing one biological replicate. Ascorbic acid content was determined by its ability to decolorize 2,6-dichlorophenol-indophenol dye, with absorbance measured at 518 nm ; .
Total carbohydrates content
Total carbohydrate content was determined in tomato fruits collected from three randomly selected plants per treatment, with each plant representing one biological replicate. Carbohydrates were quantified using the phenol-sulfuric acid method after extraction with HClO4. Absorbance was measured at 490 nm and expressed as µg glucose/g fresh weight ; .
Total soluble solids (TSS)
Total soluble solids (TSS) were determined in tomato fruit juice using a digital refractometer and expressed as °Brix, with three biological replicate per treatment. .
Total phenolics and flavonoids
Total phenolic and flavonoid contents were determined in tomato leaf tissues collected from three randomly selected plants per treatment, with each plant representing one biological replicate. Total phenolics were estimated using the Folin–Ciocalteu method , while total flavonoids were determined using the aluminium chloride colorimetric method .
Enzyme activity
Enzyme activities were determined in tomato leaf tissues obtained from three randomly selected plants per treatment (n= 3). Crude enzyme extracts were prepared from fresh leaf tissues according to several established protocols. Briefly, 1 g of fresh leaf tissue was homogenized in chilled potassium phosphate buffer (0.1 M, pH 7.0) using a pre-cooled mortar and pestle. The homogenate was centrifuged at 10,000–12,000 × g for 15–20 min. at 4 °C. The resulting supernatant was collected and used as the crude enzyme extract for subsequent biochemical assays. Polyphenol oxidase (PPO), peroxidase (PO), chitinase, and β-1,3-glucanase activities were determined using standard spectrophotometric methods as described by Ishaaya (1971); Hammerschmidt et al. (1982); Boller and Mauch (1988); Ni et al. (2001); Sun et al. (2006), respectively. Enzyme activities were expressed as activity units per gram of fresh tissue per unit time (ΔA min/ g FW), according to the respective assay procedures.
Statistical analyses
The collected data were subjected to analysis of variance (ANOVA). The treatment means were compared using the least significant difference (LSD) test at the 5% probability level (p ≤ 0.05), according to Snedecor and Cochran (1989).
Results
Isolation, purification, and identification of fungi from rotted tomato fruits
A total 85 fungal isolates recovered from rotten tomato fruits in Menoufia Governorate, Egypt, were purified and identified as A. solani and A. alternata based on their cultural, morphological and microscopic characteristics (Table 1). The findings revealed that Sadat City had the highest incidence of Alternaria spp., with recorded frequencies of 36.36 for A. solani and 40.00 for A. alternata, followed by Kafr Dawoud (33.33 and 36.00, respectively). In general, A. solani was more prevalent (33 isolate) than A. alternata (25 isolate). Consequently, Sadat City was selected as the main study site for evaluating the different eco-friendly biocontrol strategies against tomato fruit rot.
Table 1: Frequency (%) of Alternaria spp. isolated from rotten fruits of tomato collected during 2023/24 growing season.
|
Different locations |
Frequency of Alternaria spp. |
|||
|
A. solani |
A. alternata |
|||
|
No. |
(%) |
No. |
(%) |
|
|
Ashmoun district |
3 |
9.09 |
2 |
8.00 |
|
Bagour district |
7 |
21.21 |
5 |
20.00 |
|
Birkat El Sabaa district |
4 |
12.12 |
3 |
12.00 |
|
Kafr Dawood |
11 |
33.33 |
9 |
36.00 |
|
Sadat city |
12 |
36.36 |
10 |
40.00 |
|
Total |
33 |
- |
25 |
- |
Pathogenicity assessment and susceptibility evaluation of tomato cultivars to early blight disease
Data presented in Table 2 indicate that all Alternaria spp. caused typical early blight symptoms with variable disease incidence and severity among the tested tomato cultivars. A. solani was the most virulent pathogen, especially the Super strain B hybrid, which exhibited the highest disease incidence (96.3%) and severity (34.36%). In contrast, the other cultivars showed a comparatively lower susceptibility, with Super Alteray recording the lowest incidence (64.2%) and severity (15.35%) when treated with A. solani. Overall, due to the high virulence of A. solani and the high susceptibility of the Super strain B hybrid, both were selected as the model pathosystem for subsequent experiments aimed to evaluating the effective biocontrol strategies.
Table 2: Pathogenicity assessment and susceptibility evaluation of tomato cultivars to early blight disease under greenhouse conditions.
|
Different tomato cultivars (cv.) |
Sadat city |
|||
|
A. solani |
A. alternata |
|||
|
Disease incidence (%) |
Disease severity (%) |
Disease incidence (%) |
Disease severity (%) |
|
|
Super stain B hybrid |
96.3 |
34.36 |
86.0 |
43.0 |
|
Super strain Bnormal |
76.1 |
20.50 |
63.3 |
14.1 |
|
Super alteray |
64.2 |
15.35 |
49.4 |
9.3 |
|
Castel rock |
81.0 |
27.30 |
69.5 |
16.2 |
|
Elisa |
68.4 |
21.40 |
53.2 |
11.4 |
|
L.S.D.0.05 |
Cultivars (cv.)=1.29 |
Isolates (I)= 1.31 |
cv.×I= 2.62 |
|
The mean values were calculated from three randomly selected replicate for each treatment.
In vitro inhibitory potential of the selected antagonists on Alternaria solani
Data presented in Table 3 indicate the in vitro assay used to assess the antagonistic potential of several Trichoderma spp. bio-agents against the mycelial growth of A. solani, revealed that all tested antagonists substantially suppressed the fungal development with varying efficiencies. Among them, T. album exhibited the strongest inhibitory effect, achieving 90.8% growth reduction, followed closely by T. atroviride (88.72%). The commercial bio-fungicide Blight Stop (T. harzianum) displayed a moderate effectiveness (78.32%), while T. harzianum demonstrated a comparatively lower inhibition (72.18%). T. hamatum was the least effective antagonist, though it still provided a considerable reduction in fungal growth (69.16%), indicating that all bio-agents possessed varying degrees of biocontrol potential against the fungal pathogen.
Table 3: Inhibitory effects of Trichoderma spp. bio-agents on the inhibition (%) of Alternaria. solani linear growth after 5 d of incubation at 25±2°C.
|
Antagonists |
A. solani |
|
|
Linear growth (mm) |
Reduction (%) |
|
|
T. album |
8.7 |
90.28 |
|
T. atroviride |
10.1 |
88.72 |
|
T. hamatum |
27.6 |
69.16 |
|
T. harzianum |
24.9 |
72.18 |
|
Blight stop (T. harzianum) |
19.4 |
78.32 |
|
Control untreated |
89.5 |
0.00 |
|
L.S.D at 1% for: Pathogenic fungus (P) |
= 0.52 |
A×P=1.20 |
|
Antagonists (A) |
= 0.68 |
|
The mean values were calculated from three randomly selected replicate for each treatment.
Field experiments
Effect of bio-agent’s treatment on the management of tomato fruit rot under field conditions
Results presented in Table 4 reveal that all tested biological agents T. album, T. atroviride, T. harzianum, T. viride, and the commercial bio-product Blight Stop effectively reduced tomato fruit rot compared to the untreated control under field conditions during the 2023/24 and 2024/25 growing seasons. The degree of disease suppression differed among the applied treatments but remained consistent across both seasons. T. album showed the highest efficacy, achieving a disease control (%) of 73.56% and 74.76%, respectively. This was followed by T. atroviride, which also demonstrated a strong performance with 70.60% and 71.76% control. The bio-preparation Blight Stop provided a moderate disease reduction, recording 64.76% and 66.76% across the two seasons. In contrast, T. hamatum exhibited the lowest effectiveness, achieving 58.12% and 59.07% disease control only. These findings highlight the superior performance of T. album and T. atroviride as promising biocontrol agents for managing tomato fruit rot under field conditions.
Influence of biological treatments on tomato yield parameters under field trials during 2023/24–2024/25 growing seasons
The data presented in Table 5 clearly demonstrate that application of the tested antagonistic fungi and Blight Stop at a dilution of 1:50, considerably improved tomato yield parameters, with more pronounced effects observed during the 2023–2024 growing season than during the 2024/2025 season. Among the evaluated treatments, T. album exhibited the highest efficacy, markedly improving yield components, with 47.3 fruits/ plant, an average fruit weight of 104.4 g, and a total fruit yield of 4938.12 g/ plant. In contrast, T. hamatum showed the lowest improvement in yield, recording 37.1 fruits/ plant, an average fruit weight of 90.3 g, and a total fruit yield of 3729.39 g/ plant. Meanwhile, T. atroviride, Blight Stop, and T. harzianum displayed intermediate effects on yield attributes, producing 44.8, 41.3, and 39.3 fruits/ plant, with average fruit weights of 102.4, 101.0, and 95.3 g, and total fruit yields of 4587.52, 3747.10, and 3745.29 g/ plant, respectively, during the 2023/2024 growing season.
Table 4: Effect of treating tomato plants with different bio-agents under field conditions during the growing seasons (2023/24-2024/25).
|
Different treatments |
2023/24 growing season |
2024/25 growing season |
||||||
|
Disease incidence % |
Disease severity % |
Mean |
Efficacy* % |
Disease incidence % |
Disease severity % |
Mean |
Efficacy* % |
|
|
T. album |
15.4 |
4.3 |
9.85 |
73.56 |
14.2 |
4.3 |
9.25 |
74.76 |
|
T. atroviride |
16.7 |
5.2 |
10.95 |
70.60 |
15.5 |
5.2 |
10.35 |
71.76 |
|
T. hamatum |
24.1 |
7.1 |
15.6 |
58.12 |
22.9 |
7.1 |
15 |
59.07 |
|
T. harzianum |
22.5 |
7.7 |
15.1 |
59.46 |
21.3 |
7.7 |
14.5 |
60.44 |
|
Blight stop (T. harzianum) |
18.2 |
6.5 |
12.35 |
66.85 |
17.0 |
6.5 |
11.75 |
67.94 |
|
Control |
59.1 |
15.4 |
37.25 |
0.00 |
57.9 |
15.4 |
36.65 |
0.00 |
|
LSD at 5% |
2.83 |
0.88 |
2.81 |
0.88 |
||||
Where; *Efficacy of biological treatments (%) = [(Mean of Control disease parameters –Treatment)/ Mean of Control disease parameters)] ×100. The mean values were calculated from three randomly selected replicate for each treatment.
Table 5: Effectiveness of different bio-agent’s treatment applications on tomato yield parameters under field conditions during 2023/24 and 2024/25.
|
Different treatments |
2023/24 growing season |
2024/25 growing season |
||||
|
No. of fruit/ plant |
Average fruit weight/ (g/fruit) |
Fruit yield (g/plant) |
No. of fruit/ plant |
Average fruit weight/ (g/fruit) |
Fruit yield (g/plant) |
|
|
T. album |
47.3 |
104.4 |
4938.12 |
45.3 |
102.4 |
4638.72 |
|
T. atroviride |
44.8 |
102.4 |
4587.52 |
42.8 |
100.4 |
4297.12 |
|
T. hamatum |
37.1 |
90.3 |
3729.39 |
37.3 |
88.3 |
3293.59 |
|
T. harzianum |
39.3 |
95.3 |
3745.29 |
39.3 |
93.3 |
3666.69 |
|
Blight stop (T. harzianum) |
41.3 |
101.0 |
3747.10 |
41.4 |
99.0 |
4098.60 |
|
Control |
13.4 |
45.6 |
1979.04 |
10.7 |
43.6 |
466.52 |
|
LSD at 5% |
0.88 |
2.12 |
10.22 |
0.77 |
2.10 |
10.12 |
The mean values were calculated from three randomly selected replicate for each treatment.
During the 2024/2025 growing season, T. album demonstrated the highest efficacy in enhancing tomato yield components, producing the greatest number of fruits/ plant (45.3), highest average fruit weight (102.4 g), and consequently the highest total fruit yield (4638.72 g/ plant). In contrast, T. hamatum exhibited the lowest efficacy, recording 37.3 fruits/ plant, an average fruit weight of 88.3 g, and a total fruit yield of 3293.59 g/ plant. Intermediate effects were observed with T. atroviride, Blight Stop, and T. harzianum, which recorded 42.8, 41.4, and 39.3 fruits/ plant, respectively. Their corresponding average fruit weights were 100.4, 99.0, and 93.3 g, while total fruit yields reached 4297.12, 4098.60, and 3666.69 g/ plant, respectively. Overall, these findings indicate that T. album was the most effective treatment for improving the major yield attributes of tomato in the 2024/2025 growing season.
Evaluation of different biological treatments on tomato fruit quality under field conditions throughout the two growing seasons (2023/24-2024/25)
The analyses presented in Table 6 clearly indicate that all applied treatments remarkably enhanced tomato fruit quality parameters, compared to the untreated control across both 2023/2024 and 2024/2025 growing seasons. The assessed quality attributes were Total soluble solids (TSS), vitamin C content, protein content, and total carbohydrates, which are critical indicators of both the nutritional value and market acceptability of the tomato fruits. Among the tested treatments, T. album demonstrated the highest efficacy, consistently recording superior values for all measured parameters in both seasons. Specifically, TSS reached 6.7% and 4.7%, vitamin C content increased to 47.2 and 44.95 mg/100 g fresh weight (FW), protein content reached 4.35 and 4.20 g/100 g FW, and total carbohydrates were 35.82 and 33.82 mg/100 g FW during the first and second seasons, respectively. The second most effective treatment was T. atroviride, which also produced notable improvements in fruit quality. It recorded TSS values of 6.4% and 4.4%, vitamin C contents of 44.7 and 42.60 mg/100 g FW, protein levels of 3.75 and 3.60 g/100 g FW, and total carbohydrates of 34.50 and 32.50 mg/100 g FW in the two respective seasons. These obtained results suggested a strong and consistent role of certain Trichoderma species in enhancing the biochemical composition of the tomato fruits. Blight Stop (T. harzianum) ranked the third among the evaluated treatments in terms of biocontrol efficacy and also produced notable improvements in fruit quality. It recorded TSS values of 6.3% and 4.3%, vitamin C contents of 44.10 and 41.90 mg/100 g FW, protein levels of 3.40 and 3.25 g/100 g FW, and total carbohydrate contents of 33.67 and 31.67 mg/100 g FW during the 2023–2024 and 2024–2025 seasons, respectively. In contrast, T. hamatum exhibited the lowest effectiveness among the biological treatments. Overall, the current findings emphasize the superiority of T. album, followed by T. atroviride, in improving tomato fruit quality under field conditions, highlighting their potential as effective ecofriendly biostimulants in sustainable tomato production systems.
Influence of biological treatments on the activity of tomato leaf flavonoids and total phenols under field conditions during two growing seasons (2023/24–2024/25)
The data presented in Table 7 clearly display that all applied treatments considerably enhanced the accumulation of flavonoids and total phenolic
Table 6: Evaluation of the effect of different bio-agent’s treatments on tomato fruit quality under field conditions throughout two growing seasons (2023/24-2024/25).
|
Different treatments |
2023/24 growing season |
2024/25 growing season |
||||||||
|
TSS* |
Vitamin C (mg/100g FW) |
Protein (g/100g FW) |
Carbohydrate (mg/g FW ) |
TSS* |
Vitamin C (mg/100g FW) |
Protein (g/100g FW) |
Carbohydrate (mg/g FW ) |
|||
|
T. album |
6.7 |
47.2 |
4.35 |
35.82 |
4.7 |
44.95 |
4.20 |
33.82 |
||
|
T. atroviride |
6.4 |
44.7 |
3.75 |
34.50 |
4.4 |
42.60 |
3.60 |
32.50 |
||
|
T. hamatum |
6.0 |
39.8 |
2.08 |
27.97 |
4.0 |
37.90 |
1.93 |
25.97 |
||
|
T. harzianum |
6.2 |
40.6 |
2.65 |
28.85 |
4.2 |
38.53 |
2.50 |
26.85 |
||
|
Blight stop (Trichoderma spp.) |
6.3 |
44.1 |
3.40 |
33.67 |
4.3 |
41.90 |
3.25 |
31.67 |
||
|
Control |
3.7 |
20.0 |
0.85 |
14.35 |
1.7 |
18.00 |
0.70 |
12.35 |
||
|
LSD at 5% |
0.22 |
2.14 |
0.12 |
1.32 |
0.18 |
2.12 |
0.11 |
1.29 |
||
Where; *TSS: Total soluble solids. The mean values were calculated from three randomly selected replicate for each treatment.
Table 7: Influence of bio-agent’s treatments on the activity of tomato leaf flavonoids and total phenols under field conditions during the two growing seasons (2023/24–2024/25).
|
Different treatments |
2023/24 growing season |
2024/25 growing season |
||
|
Flavonoids |
Total phenols |
Flavonoids |
Total phenols |
|
|
T. album |
55.0 |
200.2 |
53.0 |
198.2 |
|
T. atroviride |
50.9 |
196.0 |
48.9 |
194.0 |
|
T. hamatum |
42.9 |
171.5 |
40.9 |
169.6 |
|
T. harzianum |
44.4 |
181.4 |
42.4 |
179.4 |
|
Blight stop (T. harzianum) |
44.9 |
186.3 |
42.9 |
184.3 |
|
Control |
30.0 |
126.0 |
28.0 |
124.0 |
|
LSD at 5% |
1.33 |
2.22 |
1.32 |
2.11 |
The mean values were calculated from three randomly selected replicate for each treatment.
compounds in tomato leaves, compared to the untreated control during both the 2023/2024 and 2024/2025 growing seasons. These biochemical parameters are key indicators of induced plant defense and antioxidant capacity. Among the tested treatments, T. album exhibited the highest stimulatory effect, recording flavonoid and total phenol contents of 55.0% and 200.20% in the first season, and 53.0% and 198.20% in the second season, respectively. This superior performance highlights its strong role in activating plant secondary metabolism and enhancing resistance mechanisms. Treatment with T. atroviride ranked the second, which showed a noticeable increase in flavonoid and total phenol contents, recording 50.9% and 196.0% in the first season, and 48.9% and 194.00% in the second season, respectively. Blight stop (T. harzianum) as a biocide came at the third effective treatment compared to the bio-agents, recording flavonoid and total phenol contents of 44.9% and 186.3% in the first season, and 42.9% and 184.30% in the second season, respectively. In contrast, the remaining treatments produced moderate improvements. T. hamatum showed the least influence on flavonoid content (42.9% and 40.9%) and phenolic accumulation (171.5% and 169.6%) during the two growing seasons 2023/24 and 2024/25, respectively. Overall, the obtained results confirmed the effectiveness of Trichoderma spp., particularly T. album, in promoting the biochemical defense responses in the treated tomato plants.
Impact of different treatments on tomato plant enzyme responses in the field throughout two growing seasons (2023/24-2024/25)
The results presented in Table 8 clearly indicate that all evaluated treatments remarkably enhanced the activities of key defense-related enzymes, mainly PO, PPO, chitinase, and β-1,3-glucanase in tomato leaves, compared to the untreated control during both 2023/2024 and 2024/2025 growing seasons. These enzymes play crucial roles in plant defense mechanisms against pathogens infection. Among the tested treatments, T. album displayed the highest activities of all the evaluated defense-related enzymes during both growing seasons, recording PO, PPO, chitinase, and β-1,3-glucanase activities of 219.00 ΔA min./ g FW, 13.25 ΔA min./ g FW, 28.50 µmol N-acetylglucosamine min./ g FW, and 5.95 µ mol glucose equivalents min./ g FW, respectively, in the first season. The corresponding activities in the second season were 217.00 ΔA min./ g FW, 11.95 ΔA min./ g FW, 27.20 µmol N-acetylglucosamine min./ g FW, and 4.92 µmol glucose equivalents min./ g FW, respectively. This superior performance reflected its strong ability to induce systemic resistance and enhance plant biochemical defenses. Treatment with T. atroviride ranked the second, exhibiting comparatively high activities of the evaluated defense-related enzymes. In the 2023/2024 season, PO, PPO, chitinase, and β-1,3-glucanase activities reached 210.00 ΔA min./ g FW, 13.06 ΔA min./ g FW, 25.90 µmol N-acetylglucosamine min./ g FW, and 5.45 µmol glucose equivalents min./ g FW, respectively. The corresponding values in 2024/2025 were 208.00 ΔA min./ g FW, 11.76 ΔA min./ g FW, 24.60 µmol N-acetylglucosamine min./ g FW, and 4.42 µmol glucose equivalents min./ g FW, respectively.
Blight Stop ranked the third among the evaluated treatments, expressing comparatively high activities of the assessed defense-related enzymes. During the 2023/2024 season, PO, PPO, chitinase, and β-1,3-glucanase activities reached 208.00 ΔA min./ g FW, 13.05 ΔA min./ g FW, 24.85 µmol N-acetylglucosamine min./ g FW, and 5.22 µmol glucose equivalents min./ g FW, respectively. In the 2024/2025 season, the corresponding activities were 206.00 ΔA min./ g FW, 11.75 ΔA min./ g FW, 23.55 µmol N-acetylglucosamine min./ g FW, and 4.19 µmol glucose equivalents min./ g FW, respectively. In contrast, T. hamatum exhibited the lowest activities of the evaluated defense-related enzymes among the tested treatments. During the 2023/2024 season, PO, PPO, chitinase, and β-1,3-glucanase activities reached 190.00 ΔA min./ g FW, 12.80 ΔA min./ g FW, 20.00 µmol N-acetylglucosamine min./ g FW, and 4.20 µmol glucose equivalents min./ g FW, respectively. The corresponding activities during the 2024/2025 season were 188.00 ΔA min./ g FW, 11.50 ΔA min./ g FW, 18.70 µmol N-acetylglucosamine min./ g FW, and 3.17 µmol glucose equivalents min./ g FW, respectively. The remaining treatments induced moderate increases in enzyme activities relative to the untreated control. Overall, these findings demonstrate the capacity of Trichoderma spp. to enhance defense-related enzymatic responses in tomato plants under field conditions, with T. album exhibiting the most pronounced stimulatory effect.
Discussion
In recent years, it has become evident that extensive use of the chemical pesticides in agriculture poses serious risks to both the environment and human health due to their high toxicity. These chemicals disrupt the natural biological balance, leading to the emergence of new pest species, cause a decline in populations of beneficial natural enemies, and the accumulation of harmful residues within the human food chain ; .
Fungal pathogen’s isolation from rotten tomato fruits in Menoufia Governorate led to the recovery of A. solani and A. alternata as the predominant pathogens, with A. solani occurring more frequently due to its stronger virulence and adaptation to tomato tissues ; . Both species are widely distributed and are the major contributors to fruit rot and postharvest losses, particularly under favourable environmental conditions such as high humidity and moderate temperatures ; ; . Previous studies confirmed the dominance of Alternaria spp. in infected tomato fruits, often representing a large
Table 8: Effect of treating tomato with bio-agents on the activity of peroxidase (PO), polyphenol oxidase (PPO), chitinase and β-1,3 glucanase enzymes under field conditions during 2023/24 and 2024/25 growing seasons.
|
Different treatments |
2023/24 growing season |
2024/25 growing season |
||||||
|
PO |
PPO |
Chitinase |
β-1,3 glucanase |
PO |
PPO |
Chitinase |
β-1,3 glucanase |
|
|
T. album |
219 |
13.25 |
28.50 |
5.95 |
217 |
11.95 |
27.20 |
4.92 |
|
T. atroviride |
210 |
13.06 |
25.90 |
5.45 |
208 |
11.76 |
24.60 |
4.42 |
|
T. hamatum |
190 |
12.80 |
20.00 |
4.20 |
188 |
11.50 |
18.70 |
3.17 |
|
T. harzianum |
203 |
12.90 |
22.50 |
4.83 |
201 |
11.60 |
21.20 |
3.80 |
|
Blight stop (T. harzianum) |
208 |
13.05 |
24.85 |
5.22 |
206 |
11.75 |
23.55 |
4.19 |
|
Control |
158 |
5.95 |
7.50 |
0.50 |
156 |
4.65 |
6.20 |
0.40 |
|
LSD at 5% |
2.62 |
0.14 |
0.24 |
0.11 |
2.44 |
0.12 |
0.22 |
0.10 |
Where: PO: Peroxidase, PPO: Polyphenol oxidase. The mean values were calculated from three randomly selected replicate for each treatment.
proportion of the fungal population ; . Their prevalence is attributed to their ecological adaptability, rapid growth, and ability to produce enzymes and mycotoxins that enhance tissue colonization and deterioration ; , highlighting the need for effective management strategies .
Pathogenicity tests of the isolated Alternaria spp. confirmed their strong virulence on tomato, typically producing early blight symptoms such as concentric leaf spots, stem lesions, and fruit rot, in consistence with the previous studies reported by Rotem (1994); Agrios (2005). These results fulfilled Koch’s postulates, verifying that these obtained isolates were the causal agents of the disease, in agreement with Chaerani and Voorrips (2006). Tomato cultivars showed a variable susceptibility, reflecting the substantial role of host genetics in disease development, as also noted by Roy et al. (2019). The resistant cultivars limit the microbial infection through several structural and biochemical defenses, while environmental factors particularly high humidity, moderate temperatures (20–30 °C), and prolonged leaf wetness may enhance the disease severity . Additionally, differences in virulence among the current isolates were observed, with A. solani generally more aggressive than A. alternata, probably due to its production of cell wall–degrading enzymes and toxins that facilitate host tissue colonization ; .
The current discussion confirmed that all tested bio-agents effectively suppressed A. solani, with Trichoderma spp. i.e. T. album, T. atroviride, T. harzianum, and T. viride demonstrated a superior biocontrol performance through multiple suggested mechanisms, including mycoparasitism, antibiosis, competition, induction of plant defense responses, and the secretion of lytic enzymes (i.e., chitinases, glucanases, proteases) and antifungal metabolites . The observed high efficacy of T. album and T. atroviride was consistent with previous studies, which displayed that Trichoderma spp. produced antifungal metabolites and cell wall-degrading enzymes, which inhibited pathogen growth and enhanced host resistance . Additionally, the relatively lower efficacy observed for T. harzianum and T. hamatum supported the concept that biocontrol efficiency is a strain-dependent and is influenced by genetic and environmental factors affecting enzyme production and adaptability . Commercial formulations such as Blight Stop displayed a moderate effectiveness, supporting their role as ecofriendly alternatives despite their slightly lower activity ; . Overall, these obtained results aligned with several previous studies emphasizing the importance of Trichoderma spp. as highly effective biocontrol agents in sustainable plant disease management ; ; .
The present field results clearly demonstrated that all tested Trichoderma spp. based treatment’s considerably reduced tomato fruit rot compared to the untreated control, confirming their effectiveness as biological control agents under natural conditions. The superior performance of T. album, which achieved the highest disease reduction across both tested seasons, may be attributed to its strong rhizosphere competence, rapid colonization, and ability to produce a wide range of antifungal metabolites . These include secondary compounds and hydrolytic enzymes that directly inhibit pathogen growth and enhance plant defense responses. Similar findings were reported by Harman (2006), who described Trichoderma spp. as highly effective biocontrol agents due to their combined mechanisms of mycoparasitism, antibiosis, and induction of systemic resistance. Furthermore, Vinale et al. (2008) emphasized that certain Trichoderma strains can stimulate plant metabolism and improve resistance against fungal pathogens under both greenhouse and field conditions.
The current obtained results indicated that all tested Trichoderma’s-based treatments remarkably improved tomato yield parameters under field conditions, with T. album expressing the highest effectiveness by enhancing fruit number, weight, and total yield. This superior performance was most likely due to its strong ability to promote plant growth, improve nutrient uptake, and suppress pathogens through multiple mechanisms ; . These findings agree with several previous studies reporting that Trichoderma spp. enhance crop productivity by stimulating plant growth and inducing resistance . Other treatments, including T. atroviride, T. harzianum, and the commercial product Blight Stop, expressed moderate and variable effects. This variation may be attributed to species- and strain-specific differences in their ability to colonize plant tissues, produce bioactive metabolites, and activate plant defense mechanisms, resulting in a differential induction of the defense-related enzymes. Benítez et al. (2004); Vinale et al. (2008) reported that the biocontrol efficacy of the Trichoderma spp. depends strongly on the type strain along with its interaction with the host plant and the pathogen. Overall, these findings support the use of biocontrol agents, particularly T. harzianum, as sustainable alternatives to chemical inputs for enhancing tomato productivity ; Ahmed et al., 2021; .
All the tested Trichoderma-based treatments, including the individual biocontrol agents and the commercial Trichoderma-based Blight Stop product, markedly improved tomato fruit quality compared to the untreated control, as evidenced by enhanced physicochemical and nutritional attributes such as TSS, vitamin C, protein content, and carbohydrate content across both seasons. T. album proved to be the most effective treatment, consistently producing the highest values for all the tested quality parameters, followed by T. atroviride. This superior performance was likely due to the ability of T. album to enhance nutrient uptake, stimulate plant metabolism, and promote the biosynthesis of secondary metabolites, which improve fruit nutritional quality and reduce pathogen pressure, allowing greater allocation of resources to fruit development ; . These findings are consistent with previous studies demonstrating that Trichoderma spp. act as plant growth promoters and biostimulants, improving both yield and fruit quality through physiological and biochemical modulation ; . Additionally, Vinale et al. (2008) reported that Trichoderma spp. can enhance plant metabolic processes and increase the accumulation of beneficial compounds in crops. The relatively lower performance of T. hamatum further confirmed that the efficiency of Trichoderma strains varies depending on their biological activity and environmental adaptability . Among treatments, T. harzianum was the most effective due to its ability to produce phytohormones and bioactive metabolites, improve nutrient availability, and stimulate antioxidant accumulation ; .
Blight Stop markedly improved tomato fruit quality compared to the untreated control, as reflected by increases in TSS, vitamin C, protein, and carbohydrate contents across both growing seasons. These improvements may be attributed to the ability of Trichoderma-based bioproducts to stimulate plant growth, nutrient acquisition, and secondary metabolism, thereby enhancing the accumulation of nutritionally important fruit constituents . Similar improvements in tomato fruit quality following Trichoderma application have been reported, including enhanced TSS and ascorbic acid, supporting the potential of Trichoderma-based products as sustainable tools for producing higher-quality tomato fruits . Overall, these findings support the roles of the tested bio-agents and Blight stop in improving tomato fruit quality in sustainable production systems.
All Trichoderma spp. and Blight stop-based treatments considerably increased flavonoid and total phenolic contents in tomato leaves compared to the untreated control, indicating an enhanced plant defense and antioxidant capacity across both seasons. T. album showed the strongest stimulatory effect, followed by T. atroviride, while T. hamatum was the least effective. The elevated accumulation of these secondary metabolites suggested the activation of plant defense pathways and improved resistance to stress. These findings are consistent with previous studies demonstrating that Trichoderma spp. can induce systemic resistance and stimulate the production of phenolics and flavonoids as part of plant defense mechanisms ; . This enhancement in flavonoid and total phenolic contents was linked to the activation of plant defense mechanisms, as these secondary metabolites function as antioxidants and antimicrobial compounds that improve stress tolerance ; . Among treatments, T. harzianum displayed the highest effect due to its ability to induce systemic resistance and stimulate the phenylpropanoid pathway via activation of defense enzymes such as phenylalanine ammonia-lyase (PAL) ; ; ; .
All the presently evaluated Trichoderma spp. and Blight stop-based treatments substantially enhanced the activities of key defense-related enzymes, mainly PO, PPO, chitinase, and β-1,3-glucanase in tomato leaves, compared to the untreated control across both growing seasons. T. album demonstrated the highest enzyme induction, followed by T. atroviride, while T. hamatum showed the lowest activity. The increased levels of these enzymes indicated the activation of several plant defense mechanisms, including strengthened cell walls, degradation of pathogen cell components, and enhanced resistance to infection. These obtained results are consistent with previous findings reporting that Trichoderma spp. induce systemic resistance by stimulating defense-related enzymes and biochemical pathways ; ; .
Conclusions and Recommendations
This study demonstrated the potential of integrated, eco-friendly biocontrol strategies for managing tomato fruit rot while improving yield, fruit quality, and plant defense responses. Among the isolated pathogens, Alternaria solani was more prevalent and virulent than A. alternata, causing a severe disease in the tomato Super Strain B hybrid, recording 96.30% incidence and 34.36% severity. All evaluated Trichoderma spp. and the commercial Trichoderma-based product Blight Stop exhibited a substantial antagonistic activity against A. solani, both in vitro and in vivo. T. album showed the greatest biocontrol efficacy, achieving 90.28% mycelial growth inhibition in vitro and 73.56–74.76% disease-control efficiency across the 2023/2024 and 2024/2025 growing seasons, respectively. Moreover, T. album consistently produced the greatest improvements in yield components, TSS, vitamin C, protein content, carbohydrates, flavonoids, total phenolics, and defense-related enzymes, including PO, PPO, chitinase, and β-1,3-glucanase. Overall, these findings confirm that Trichoderma spp., particularly T. album, represent promising sustainable and environmentally compatible alternatives to the conventional fungicides used for suppressing tomato fruit rot pathogen, and simultaneously enhance crop productivity, fruit nutritional quality, and innate defense capacity under field conditions. Based on the present findings, T. album is recommended as a promising eco-friendly biocontrol agent for the integrated management of tomato fruit rot caused by Alternaria solani. Its superior disease-suppressive activity, along with its positive effects on yield, fruit quality, and plant defense responses, recommends its potential as a sustainable alternative to the conventional fungicides.
Acknowledgement
Not applicable.
Novelty Statement
This study presents an integrated approach combining biological control agents and the bioproduct Blight Stop as ecofriendly alternatives to chemical pesticides used for the management of tomato diseases and improves tomato fruit quality and safety for human use.
Authors’ Contributions
MFAA: Conceptualization, methodology, validation, investigation, resources, writing original draft, writing review and editing, visualization, project administration, and supervision.
HHY: Conceptualization, methodology, validation, investigation, resources, writing review and editing, visualization, and funding acquisition.
MAE-A: Methodology, formal analysis, investigation, data curation, writing original draft, writing review and editing, and visualization.
MMY: Software, data curation, and writing review and editing.
AAE: Writing original draft, statistical analysis, and writing review and editing.
All authors have read, critically reviewed, and approved the final version of the manuscript for publication.
Funding source
This study did not receive any fund.
Ethical approval
None applicable.
Generative AI and AI assisted technology statement
The authors declare that no generative AI and AI assisted technology was used in the creation of this manuscript.
Conflict of interests
The authors have declared no conflicts of interest.
Figures
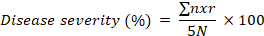
References
- AOAC, 2005. Official methods of Analysis of AOAC International. 18th ed. W. Horwitz and G.W. Latimer Jr. (Eds.). AOAC International, Gaithersburg, MD, USA, pp. 10-12.
- Agrios, G.N., 2005. Plant pathology. 5th Edition. Elsevier Academic Press, London, New York, pp. 922.
- Ahmed, M.F.A., 2005. Effect of adding some biocontrol agents on non-target microorganisms in root diseases infecting soybean and broad bean plants. M.Sc. Thesis. Fac. Agric., Moshtohor, Benha Univ., pp. 137.
- Ahmed, M.F.A., 2013. Studies on non-chemical methods to control some soil borne fungal diseases of bean plants Phaseolus vulgaris L. Ph.D. Thesis. Fac. Agric., Cairo Univ., Egypt, pp. 137.
- Ahmed, M.F.A., Ahmed, M.S.M. and Mervat, G.AE-A., 2021. Influence of biological control on sweet pepper powdery mildew disease and its impact on growth and yield under greenhouse condition. Future J. Agric., 3: 52-63. https://doi.org/10.37229/fsa.fja.2021.08.18[CrossRef]
- Ahmed, M.F.A., Ali, A.A.M. and Shaheen, S.I., 2023. Efficacy of some biological control treatments on grey mold disease (Botrytis cinerea) of strawberry fruits. J. Plant Prot. Path., Mansoura Univ., 14(11): 345-351. https://doi.org/10.21608/jppp.2023.242510.1187[CrossRef]
- Ahmed, M.F.A., Ali, A.A.M. and Shahin, S.I., 2022. Efficiency of some organic matter on suppression of soil-borne diseases of tomato plants under organic agriculture system. Egypt. J. Phytopathol., 50(2): 124-137. https://doi.org/10.21608/ejp.2022.172753.1074[CrossRef]
- Ahmed, M.F.A., Amin, M.M. and El-Fiki, I.A.I., 2017. Efficacy of bioagents against Alternaria porri incitant of purple blotch of onion in Egypt. Egypt. J. Phytopathol., 45(1): 17-29. https://doi.org/10.21608/ejp.2017.89518[CrossRef]
- Akila, A.H., Ali, M.A.S., Khairy, A.M., Elnahal, A.S.M., Alfassam, H.E., Rudayni, H.A., Jaber, F.A. and Tohamy, M.R.A., 2024. Biological control of tomato bacterial leaf spots and its impact on some antioxidant enzymes, phenolic compounds, and pigment content. Biology, 13(6): 369. https://doi.org/10.3390/biology13060369[CrossRef]
- Arafa, M., Shaheen, S., Mansour, A.M.K. and Ahmed, M.A., 2022. Effect of compost on root rot disease management to increase tomato plant productivity. Int. J. Environ. Stud. Res., 1(2): 250–261. https://doi.org/10.21608/ijesr.2022.296779[CrossRef]
- Barnett, H.J. and Hunter, B.B., 1987. Illustrated genera of imperfect fungi. Burgess, Publ. Co., Minneapolis, USA, pp. 218.
- Benítez, T., Rincón, A.M., Limón, M.C. and Codón, A.C., 2004. Biocontrol mechanisms of Trichoderma strains. Int. Microbiol., 7: 249–260.
- Bessadat, N., Hamon, B., Henni, J.E. and Simoneau, P., 2017. Alternaria species associated with early blight epidemics on tomato and other Solanaceae crops in northwestern Algeria. Eur. J. Plant Pathol., 148: 181–197. https://doi.org/10.1007/s10658-016-1081-9[CrossRef]
- Boller, T. and Mauch, F., 1988. Chitinase from Phaseolus vulguris, leaves. Meth. Enzymol, 161: 479-484. https://doi.org/10.1016/0076-6879(88)61062-7[CrossRef]
- Bradford, M.M., I976. A rapid and sensitive method for the quantitation of microgram quantities of proteins utilizing the principle of protein-dye binding. Anal. Biochem., 72: 248-254. https://doi.org/10.1016/0003-2697(76)90527-3[CrossRef]
- Chaerani, R. and Voorrips, R.E., 2006. Tomato early blight (Alternaria solani): The pathogen, genetics, and breeding for resistance. J. Gen. Plant Pathol., 72(6): 335–347. https://doi.org/10.1007/s10327-006-0299-3[CrossRef]
- Crompton, M. and Birt, L.M., 1967. Changes in the amounts of carbohydrates, phosphagen and related compounds during the metamorphosis of the blowfly, Lucilia cuprina. J. Insect Physiol., 13: 1575-1595. https://doi.org/10.1016/0022-1910(67)90180-1[CrossRef]
- Daraban, G.M., Hlihor, R.M. and Suteu, D., 2023. Pesticides vs. Biopesticides: From pest management to toxicity and impacts on the environment and human health. Toxics, 11(12): 983. https://doi.org/10.3390/toxics11120983[CrossRef]
- DeMers, M., 2022. Alternaria alternata as endophyte and pathogen. Microbiology, 168(3): 001153. https://doi.org/10.1099/mic.0.001153[CrossRef]
- Dubios, M., Gilles, K.A., Hamilton, J.K., Rebers, P.A. and Smith, F., 1956. Colorimetric method for determination of sugars and related substances. Anal. Chem., 28: 350-356. https://doi.org/10.1021/ac60111a017[CrossRef]
- El-Khalifa, Z., Ayoub, A. and Zahran, H., 2022. Estimating the efficiency of summer tomatoes production: A case study in Borg El-Arab area, Egypt. Open J. Appl. Sci., 12: 855–864. https://doi.org/10.4236/ojapps.2022.126058[CrossRef]
- El-Tanany, M.A., Haggag, W.M. and Hassan, H.S. 2018. Role of some defense-related enzymes in the induced systemic resistance of tomato plants against early blight disease. Egypt. J. Biol. Pest Contr., 28: 65.
- Food and Agriculture Organization of the United Nations (FAO). 2024. The State of Food and Agriculture: Value-driven transformation of agrifood systems. Rome, Italy: FAO., pp. 136.
- García-Latorre, C., Ruiz-Moyano, S., Rodríguez, A.N., Velázquez, R., Poblaciones, M.J., and Hernández, A., 2025. From field to fork: The benefits of Trichoderma spp. in food quality and safety. Curr. Opin. Food Sci., 63: 101286. https://doi.org/10.1016/j.cofs.2025.101286[CrossRef]
- Gherbawy, Y., Hussein, M.A., Runge, F. and Spring, O., 2018. Molecular characterization of Alternaria alternata population isolated from Upper Egyptian tomato fruits. J. Phytopathol., 166(10): 709–721. https://doi.org/10.1111/jph.12752[CrossRef]
- Habib, W., Masiello, M., El Ghorayeb, R., Gerges, E., Susca, A., Meca, G., Quiles, J.M., Logrieco, A.F. and Moretti, A. 2021. Mycotoxin profile and phylogeny of pathogenic alternaria species isolated from symptomatic tomato plants in Lebanon. Toxins, 13(8): 513. https://doi.org/10.3390/toxins13080513[CrossRef]
- Hajji, H.L., Rhouma, A., Wannassi, T., Utkina, A.O. and Rebouh, N.Y., 2025. Biocontrol assessment of Trichoderma species on tomato crops infested by Curvularia spicifera: Toward sustainable farming systems. Front. Sustain. Food Syst., 9: 1627903. https://doi.org/10.3389/fsufs.2025.1627903[CrossRef]
- Hammerschmidt, R., Nuckles, F. and Kuc, J., 1982. Association of enhanced peroxidase activity with induced systemic resistance of cucumber to Colletotrchum lagenarium. Physiol. Plant Pathol., 20: 73-82. https://doi.org/10.1016/0048-4059(82)90025-X[CrossRef]
- Harman, G.E., 2006. Overview of mechanisms and uses of Trichoderma spp. Phytopathol., 96(2): 190–194. https://doi.org/10.1094/PHYTO-96-0190[CrossRef]
- Harman, G.E., 2024. Integrated benefits to agriculture with Trichoderma and other endophytic or root-associated microbes. Microorganisms, 12(7): 1409. https://doi.org/10.3390/microorganisms12071409[CrossRef]
- Harman, G.E., Doni, F., Khadka, R.B. and Uphoff, N., 2021. Endophytic strains of Trichoderma increase plants’ photosynthetic capability. J. Appl. Microbiol., 130(2): 529–546. https://doi.org/10.1111/jam.14368[CrossRef]
- Harman, G.E., Howell, C.R., Viterbo, A., Chet, I. and Lorito, M., 2004. Trichoderma species-opportunistic, avirulent plant symbionts. Nat. Rev. Microbiol., 2: 43-56. https://doi.org/10.1038/nrmicro797[CrossRef]
- Hermosa, R., Viterbo, A., Chet, I. and Monte, E., 2012. Plant-beneficial effects of Trichoderma and of its genes. Microbiol., 158(1): 17–25. https://doi.org/10.1099/mic.0.052274-0[CrossRef]
- Iqbal. O., Li, C., Ahmed Rajput, N. and Mubeen Lodhi, A., 2023. Management of phytopathogens by antagonistic Bacillus spp. in tomato crop. In: F. Lops (Ed.), tomato cultivation and consumption– innovation sustainability and health, pp. 1–26. https://doi.org/10.5772/intechopen.112439[CrossRef]
- Ishaaya, I., 1971. In the armored scale Aonidiella aurantii and Observation on the phenoloxidase system Chrysomphalus aonidum. Comp. Biochem. Physiol., 39(B): 935-943. https://doi.org/10.1016/0305-0491(71)90117-9[CrossRef]
- Karačić, V., Miljaković, D., Marinković, J., Ignjatov, M., Milošević, D., Tamindžić, G. and Ivanović, M., 2024. Bacillus species: Excellent biocontrol agents against tomato diseases. Microorganisms, 12(3): 457. https://doi.org/10.3390/microorganisms12030457[CrossRef]
- Karthika, S., Varghese, S. and Jisha, M.S., 2020. Exploring the efficacy of antagonistic rhizobacteria as native biocontrol agents against tomato plant diseases. 3 Biotech., 10(7): 306. https://doi.org/10.1007/s13205-020-02306-1[CrossRef]
- Khaskheli, M.A., Khan, S. and Tunio, S.H., 2021. Postharvest losses and occurrence of Alternaria rot in tomato fruits at different marketing levels. Turk. J. Agric. Food Sci. Technol., 9(2): 288–295. https://doi.org/10.24925/turjaf.v9i2.288-295.3798[CrossRef]
- Kumar, S., Kaushik, N. and Edrisi, S.A., 2017. Role of Trichoderma spp. in improving plant growth and quality. J. Appl. Microbiol., 123(1): 1–12.
- Latha, P., Anand, T., Ragupathi, N., Prakasam, V. and Samiyappan, R., 2009. Antimicrobial activity of plant extracts and induction of systemic resistance in tomato plants by mixtures of PGPR strains and Zimmu leaf extract against Alternaria solani. Biol. Contr., 50(2): 85-93. https://doi.org/10.1016/j.biocontrol.2009.03.002[CrossRef]
- Lattanzio, V., Lattanzio, V.M.T. and Cardinali, A., 2006. Role of phenolics in the resistance mechanisms of plants against fungal pathogens and insects. In: Imperato, F. (Ed.), Phytochemistry: Advances in Research. Research Signpost, Trivandrum, Kerala, India, pp. 23–67.
- Liu, W., Yu, K., He, T., Li, F., Zhang, D. and Liu, J., 2022. Solanum lycopersicum: A model plant for studying plant development and stress responses. Front. Plant Sci., 13: 948090.
- Naik, M.K., Prasad, Y., Bhat, K.V. and Rani, G.S., 2010. Morphological, Physiological, Pathogenic and molecular variability among isolates of Alternaria solani from tomato. Indian Phytopthol., 63: 168-173.
- Nazarbekova, S.T., Alimzhanova, M. and Yerzhanov, K., 2025. Identification and characterization of Alternaria species causing early blight on tomato in Kazakhstan. Agronomy, 15(5): 1251. https://doi.org/10.3390/agronomy15051251[CrossRef]
- Ni, X., Quisenberry, S.S., Heng-Moss, T., Markwell, J., Sarath, G., Klucas, R. and Baxendale, F., 2001. Oxidative responses of resistant and susceptible cereal leaves to symptomatic and nonsymptomatic cereal aphid (Hemiptera: Aphididae) feeding. J. Econ. Entomol., 94: 743-751. https://doi.org/10.1603/0022-0493-94.3.743[CrossRef]
- Offor, P.O., Obi, C.G. and Ezeonu, C.S., 2015. Determination of phosphite in plant tissues using spectrophotometric methods. J. Appl. Chem., 8(3): 45–51.
- Pieterse, C.M.J., Zamioudis, C., Berendsen, R.L., Weller, D.M., Van Wees, S.C.M. and Bakker, P.A.H.M., 2014. Induced systemic resistance by beneficial microbes. Annu. Rev. Phytopathol., 52: 347–375. https://doi.org/10.1146/annurev-phyto-082712-102340[CrossRef]
- Poly, S. and Srikanta, D., 2022. Development of prediction equations for early blight leaf spot on tomato under different fungicides treatments. J. Agrometeorol., 16(1): 130–136. https://doi.org/10.54386/jam.v16i1.1498[CrossRef]
- Ramezani, M., Taheri, P. and Mamarabadi, M., 2024. Identification and characterization of Alternaria species associated with tomato fruit rot and their sensitivity to fungicides. J. Plant Pathol., 106: 123–135.
- Razdi, M.P.M.F., Azizah, M., Maininah, T. and Sumaiyah, A., 2021. Occurrence of tomato early blight disease and associated Alternaria species in Punjab, Pakistan. J. Anim. Plant Sci., 31(6): 1699–1711. https://doi.org/10.36899/JAPS.2021.5.0337[CrossRef]
- Reddy, P.P., 2016. Sustainable Crop Protection under Integrated Pest Management. Singapore: Springer. pp. 1–409. https://doi org/10.1007/978-981-10-2702-4.
- Rice-Evans, C., Miller, N.J. and Paganga, G., 1996. Structure–antioxidant activity relationships of flavonoids and phenolic acids. Free Radic. Biol. Med., 20(7): 933-956. https://doi.org/10.1016/0891-5849(95)02227-9[CrossRef]
- Rotem, J., 1994. The genus Alternaria spp.: Biology, epidemiology, and pathogenicity. St. Paul, MN, USA: APS Press. pp. 326.
- Roy, C.K., Akter, N., Sarker, D., Alam, M.S, Akhter, M.S. and Islam, R., 2019. Control of early blight of tomato caused by Alternaria solani and screening of tomato varieties against the pathogen. Open Microbiol. J., 13: 41–50. https://doi.org/10.2174/1874285801913010041[CrossRef]
- Schmey, T., Tominello‐Ramirez, C.S., Brune, C. and Stam, R., 2024. Alternaria diseases on potato and tomato. Mol. Plant Pathol., 25(3): e13435. https://doi.org/10.1111/mpp.13435[CrossRef]
- Shi, T., Liu, Y., Zheng, X., Hu, K., Huang, H., Liu, H. and Huang, H., 2023. Recent advances in plant disease severity assessment using convolutional neural networks. Sci. Rep., 13(1): 2336. https://doi.org/10.1038/s41598-023-29230-7[CrossRef]
- Shoresh, M., Harman, G.E. and Mastouri, F. 2010. Induced systemic resistance and plant responses to fungal biocontrol agents. Annu. Rev. Phytopathol., 48: 21–43. https://doi.org/10.1146/annurev-phyto-073009-114450[CrossRef]
- Simmons, E.G., 2007. Alternaria: An identification manual. CBS Biodiv. Ser., 6: 1-775.
- Singh, R.S., 1982. Plant Pathogens “The Fungi” Oxford and IBH publishing Co. New Delhi, Bombay Calcuta. pp. 443.
- Singh, V., Kabdwal, B.C., Sharma, R. and Tewari, R., 2019. Field efficacy of different combinations of Trichoderma harzianum, Pseudomonas fluorescens, and arbuscular mycorrhiza fungus against major diseases of tomato. Egypt. J. Biol. Pest Contr., 29(1): 1. https://doi.org/10.1186/s41938-018-0103-7[CrossRef]
- Singleton, V.L., Rosa, R.O. and Lamuela-Raventós, M., 1999. Analysis of total phenols and other oxidation substrates and antioxidants by means of Folin-Ciocalteau reagent. Methods Enzymol., 299: 152-178. https://doi.org/10.1016/S0076-6879(99)99017-1[CrossRef]
- Snedecor, G.W. and Cochran, W.G., 1989. Statistical methods, 8th edition. Iowa State Univ. Press, Ames, Iowa USA, pp. 503.
- Sun, H., Yang, J., Lin, C., Huang, X., Xing, R. and Zhang, K.Q., 2006. Purification and properties of a β-1, 3-glucanase from Chaetonium sp. that is involved in mycoparasitism. Biotechnol. Lett., 28: 131-135. https://doi.org/10.1007/s10529-005-5132-0[CrossRef]
- Thomidis, T., Prodromou, I., Paresidou, M. and Damos, P., 2023. Effects of temperature and leaf wetness duration on pathogens causing preharvest fruit rots on tomato. J. Plant Pathol., 105: 1431–1448. https://doi.org/10.1007/s42161-023-01443-9[CrossRef]
- Thomma, B.P.H.J., 2003. Alternaria spp.: From general saprophyte to specific parasite. Mol. Plant Pathol., 4(4): 225-236. https://doi.org/10.1046/j.1364-3703.2003.00173.x[CrossRef]
- Tigchelaar, E.C., 1986. Tomato breeding. In: Basset MJ. Breeding vegetables Crops. pp. 135-171.
- Tsolakidou, M.D., Demetriou, G., Panagiotou,. S, Vassiliou, L., Goulas, V. and Pantelides, I., 2024. Efficacy of commercial biocontrol products for the management of verticillium and fusarium wilt in greenhouse tomatoes: Impact on disease severity, fruit yield, and quality. Agriculture, 14(6): 882. https://doi.org/10.3390/agriculture14060882[CrossRef]
- Venkatesan, U., and Muniyan, R., 2024. Review on the extension of shelf life for fruits and vegetables using natural preservatives. Food Sci. Biotechnol., 33: 2477–2496. https://doi.org/10.1007/s10068-024-01602-3[CrossRef]
- Vinale, F., Sivasithamparam, K., Ghisalberti, E.L., Marra, R. and Lorito, M., 2008. Trichoderma- plant pathogens interactions. Soil Biol. Biochem., 40(1): 1-10. https://doi.org/10.1016/j.soilbio.2007.07.002[CrossRef]
- Vukelić, I.D., Prokić, L.T., Racić, G.M., Pešić, M.B., Bojović, M.M., Sierka, E.M., Kalaji, H.M. and Panković, D.M., 2021. Effects of Trichoderma harzianum on photosynthetic characteristics and fruit quality of tomato plants. Int. J. Mol. Sci., 22(13): 6961. https://doi.org/10.3390/ijms22136961[CrossRef]
- Yao, X., Guo, H., Zhang, K., Zhao, M., Ruan, J. and Chen, J. 2023. Trichoderma and its role in biological control of plant fungal and nematode disease. Front. Microbiol., 14:1160551. https://doi.org/10.3389/fmicb.2023.1160551[CrossRef]
- Zhang, Y., Geng, L., Fu, Y., Zhao, J. and Zhang, H., 2022. Biocontrol potential of Trichoderma harzianum against Botrytis cinerea in tomato plants. Biol. Contr., 174: 105019. https://doi.org/10.1016/j.biocontrol.2022.105019[CrossRef]
- Zhu, Y., Li, M., Wang, X. and Zhang, L., 2023. Insights into the molecular mechanisms of Alternaria alternata pathogenesis in postharvest tomato fruits. Postharv. Biol. Technol., 195: 112140.
Services
Article usage statistics
Loading…